Research Report
Preliminary ecosystem relationships of whale shark growth rates and production associated with zooplankton at seamounts and the island mass effect upwelling 
 Author
 Correspondence author
International Journal of Marine Science, 2026, Vol. 16, No. 5
Received: 15 Sep., 2026 Accepted: 15 Oct., 2026 Published: 28 Oct., 2026
The main objectives of the study are that as whale sharks are planktivorous fish, they migrate over long distances in tropical areas of the world to find zooplankton food generated at seamounts and by the island mass effect where upwelling promotes ecosystem production. Whale shark occurrence in the six main areas are discussed systematically in terms of the various causes of elevated zooplankton by processes such as upwelling by the Indo-Pacific throughflow (ITF) currents around the Indonesian islands and far-field effects on the Indian ocean to Africa. That encouraged investigation of sustainable management of the six main accumulation areas in Southwestern Taiwan, two areas in Indonesia, Caribbean Sea, Ningaloo at Eastern Indian Ocean, Western Australia and Galapagos, Ecuador, eastern Pacific Ocean, particularly the Indonesian and Galapagos breeding areas. Hence, whale shark relationships are investigated for weight with total length, and age in years with average total length and weight estimated by the innovative doubling time method using Ecopath model fish production characteristics. That gave similar results with published growth rates, including the von Bertalanffy equation, because the Ecopath model ecosystem conditions reasonably described the whale shark growth rates. The reported and expected migrations in the tropical Atlantic, Pacific and Indian Oceans are described, leading to suggested further research on whale shark production. Furthermore, due to the amount of food energy spent looking for food, the ecosystem conditions indicated their biomass and biological production are too low to support fishing, so it was suggested all whale sharks be protected.
1 Introduction
The Whale shark (Rhincodon typus) is a fish and the world’s largest planktivore. The whale shark feeding study by Motta et al. (2010), found a small juvenile of 4.43 m consumed about 11.0 kg/day of zooplankton and a large juvenile 6.22 m total length about 20.7 kg/day for a typical 7.5 hours feeding per day. They noted from the literature whale sharks are known to eat a variety of zooplankton as well as small squid and fish. They tend to move between the Tropic of Cancer, about 23.5° North, and the tropic of Capricorn, 23.436° South of the equator, wherever high upwelling promotes phytoplankton and the resulting zooplankton production that supports their mostly zooplankton diet (Ainsworth et al., 2007). As noted by Hodgson (2025), baleen whales migrate along productive west coast of continental areas due to upwelling of nutrients on their way to breeding grounds. The migration map in Horton et al. (2022) shows they migrate following the mid-Atlantic Ridge seamounts where upwelling promotes ecosystem production. In the Pacific ocean, they migrate along the west coast of North America to Mexico and the west coast of South America to southern Ecuador, Likewise, adult female whale sharks accumulate at the Galapagos Islands off Ecuador (Acuña-Marrero et al., 2014), formed by the Galapagos Rise and the deep sea Cocos ridge connecting with the west coast of South America (Robalino-Mejía et al., 2026). Later, Womersley et al. (2025) noted Darwin Island and the Wolf-Darwin volcanic ridge are volcanic seamounts in the northern Galapagos where adult female whale sharks aggregate. Hence, it was suggested the Galapagos seamounts were used for breeding and release the neonate pups for feeding and rapid growth on the abundant zooplankton, promoted by nutrients in upwelling at the seamounts (Genin, 2004), as well as providing zooplankton for the adult planktivores.
In the southern hemisphere, whale migration was noted by Hodgson (2025) along Western Australia, in the eastern Indian Ocean, likely starting from the Antarctic, and then along the archipelagos and range of islands at Ashmore, Cartier and then north into the Banda Sea around Timor and Suva, Indonesia. Whale sharks also occur in relatively large numbers at The Ningaloo marine park, Western Australia, (Norman and Stevens, 2007) where upwelling process by the Ningaloo and Leeuwin Currents increase zooplankton production (Vanderklift et al., 2020). Consequently, the aim of this paper is to investigate ecosystem relationships of whale sharks with zooplankton at seamounts and tropical islands.
2 Methods
The ecosystem relationships of whale sharks for total length with weight, age in years with weight and age with length were estimated using six independent data bases obtained from the published literature. The six whale shark areas have data on the range of total length (cm. or metres) and weight (kilograms), as well as areas (km2), varying from newborn neonate pups to juveniles, sub-adults and adults that were obtained from the references shown in Table 1. The biomass per square kilometre in each study area used by the whale sharks was estimated from reported or estimated population number, N, multiplied by the average weight, W, divided by the estimated area occupied by whale sharks in the study area, A (km2) by the equation:
|
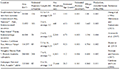
Table 1 Whale shark estimated ecosystem parameters for total length, average weight, ecosystem biomass, production to biomass ratio and production for newborn neonates to small Juvenile, large juvenile, sub-adult and adults in six representative study areas Notes: a) Southwest Taiwan 300 Newborn neonates with reported total lengths and average weight. Number of adult females assumed similar Galapagos by area, estimated number 156. The biomass was estimated as 0.001 tww/Km2 (See Methods). Fishery area 50 000 km2 (China Blue Sustainability Institute, 2018. Shantou-Taiwan Bank Fishing Ground Squid Fishery Improvement Project (FIP) Workplan (https://fisheryprogress.org/system/files/documents_workplan/Chinese%20Common%20Squid%20FIP%20workplan2018Dec-2019Dec-fin-HYL-HH.pdf) b) Cenderawasih, 15 Small juveniles sampled in the 13,851 km2 Teluk Cenderawasih National Park (https://en.wikipedia.org/wiki/Teluk_Cenderawasih_National_Park) The bay area estimated about 95 000 km2 from scaled map in Cenderawasih Bay (https://en.wikipedia.org/wiki/Cenderawasih_Bay#References) The expected average whale shark total length was 3.2 m giving average weight 450 kg by equation 2 c) Raja Ampat Large juveniles P/B taken as 1.100 from Ainsworth et al., 2007 Ecopath model for large juvenile fish. Expected average total length 5.5 m, giving average weight 2 500 kg by equation 2. Using Hueter et al. (2013) 0.666 3 x maximum total length 8 m average gave average total length 5.33 m, reducing average, weight 2 300 kg increasing P/B to 1.196 for smaller size. Study area estimated 46 000 km2 from Pitcher et al. (2007) 143t in area for biomass 0.003 t/km2 giving area ~ 46 000 km2 d) Yucatan Larger juveniles, Reported number sampled in Gulf of Mexico 728 with are a about 1 million km2 compared Yucatan reported area 116 257 km2, giving 85. Expected average total length 5.5 m gave average biomass 2 500 kg for P/B 1.100, Hueter et al. (2013) reported average total length 6.33 m giving biomass of 3 907 kg compared 2 500 kg decreased P/B to 0.704=1.1*2500/3907 e) Sub-adult at Ningaloo marine park coral reef and open shelf water areas about 4,000 km2 in southern Exmouth Plateau 280 000 km2, total area occupied by whale sharks 284 000 km2. Number assumed related to larger juveniles at Yucatan, 208 = 85*284000/116257. The reported average total length 7.3 m by Norman and Stevens (2007) gives weight 6 063 kg by equation 2. Then biomass 0.004 = ((5800*208)/284000)/1000 tww/km2 f) Galapagos Breeding, fully mature adult females. Atkinson et al. (2007) appears to assume whale sharks at Raja Ampat were breeding and tentatively set a low P/B of 0.068, but a recent study shows it applies to Galapagos whale sharks. Area occupied by whale sharks less than National Park at 26 300 km2, estimated from Acuña-Marrero et al. (2014) Reported number adult females 82. Acuña-Marrero et al. (2014) Figure 4 Size-frequency distribution female whale sharks 9.0 to 13.1 to 14.0 m, estimated average 11.0 m giving average weight 21 444 kg by equation 2 g) Cumulative age in years to reach average weight increase |
Biomass, B (tww/km2) = (N × W)/A (1)
Initially, that data and information was used to estimate the relationship of average weight with average total length. The relationship for average weight with average total length obtained was calculated using the reported newborn neonate pups average total length of 0.5 m and average weight of 1.5 kg, giving the power relationship:
Weight = 13.264 × L3.0811 ± 0.045 kg (2)
The relationship was tested using the reported average lengths, L, for the other five areas and gave a similar overall power relationship in Figure 1 (Results section). Note the total length is shown as L rather than TL to avoid confusion with the Ecopath model trophic level (TL). That was followed by estimation of the increase in age in years with average total length. Traditionally, the relationship for length with time is estimated by the von Bertalanffy (1938) growth function for human weight increase, defined as a growth curve by equation: L(t) = L∞(1 – e-K(t-to)), where L(t) represents the expected length at age time t, by the asymptotic maximum length, L∞, and growth coefficient, K, with time offset to. However, those model values are not well known (Wintner, 2000). Hence, as an alternative, the innovative doubling time method by Heip (1972) was used here. The important information on fisheries, Fishbase (https://www.fishbase.se/manual/key%20facts.htm) shows Estimation of Life-History Key Facts, and under “Intrinsic rate of population increase” states that without fishing effects, the time (td) in years that it would take a reduced population of fish to double in numbers can be estimated by td = ln(2)/r, where r is the intrinsic rate of natural increase. The r value for a fishery was shown by Hodgson (2024) using the Ecopath model P/B value by r = ln (P/B + 1). Note that the P/B values used to estimate the r values were assumed related to Ecopath models for fish, varying from larvae, juveniles, sub adults and adults. Therefore, the increase in age (years) of whale sharks with average total length in the six study areas, beginning with newborn neonate pups at age zero years, was estimated using the doubling time method described below. The results are compared with the von Bertalanffy (1938) curve in the Discussion. Note that the von Bertalanffy growth curve for length with time is a saturating growth curve, with a rapid initial increase and slowing down gradually as the human growth model, applied to animals, grows larger over time. Examples of the von Bertalanffy growth curve applied to fish are also shown in the Fishbase link.
|
Figure 1 Power relationship between whale shark average weights with average total length (L) from data in Table 1. The highest length and weight is for adult females |

2.1 Whale shark population and biomass
The assumptions and methods for estimation of the population number and biomass in each area are described here, which are briefly described in Table 1 footnotes. In some cases, the number per km2 and area occupied by whale sharks was estimated using data and information from independent locations in the literature. Additionally, average lengths and P/B ratios for each size of whale sharks in each study area was estimated using independent data and information from associated references, as described here and shown in Table 1. The results were tested by comparison for consistent relationships in graphs of the data (see Figure 1, Figure 2, Figure 3, Figure 4 in the Results section).
|
Figure 2 Exponential relationship between estimated whale shark cumulative ages in years, to reach the average total length (L) newborn neonate pups to adult females |

|
Figure 3 Linear relationship whale shark cumulative age (years) with average weight (kg) from newborn neonate pups to the next stage. As the newborn neonates have an age of zero years, it is lower than the regression for the other stages |

|
Figure 4 Linear relationship whale shark cumulative age (years) with average weight (kg) from small juveniles in Cenderawasih Bay, Indonesia to adult females at Galapagos, Ecuador |

(i) Southwestern Taiwan fishery area reported as 50 000 km2 from reliable online reference in notes to Table 1. The population number per km2 was assumed similar to the numbers at the Galapagos National Park. At Southwestern Taiwan, where 300 newborn neonates (age zero years) were reported, a population of adult female whale sharks were breeding. At the Galapagos National Park, Ecuador a large number of pregnant adults were probably soon to breed, so the number in the Park area of about 82 was estimated from the study by Acuña-Marrero et al. (2014) and used to estimate the Taiwan population of by relative proportions: 156 = (82 x Taiwan area 50 000 km2/estimated Galapagos area occupied by whale sharks 26,300 km2 rather than the park area Park area of 133 000 km2. Assuming the Taiwan population may all eventually breed by releasing the same 300 neonates during the period of high zooplankton abundance, and with the reported average neonate pup weight od 1.5 kg, the expected neonate biomass was estimated by Biomass (tww/km2) = (((1.5 kg*300*156)/1 000 convert to t/km2))/50 000 km2. Note: the biomass is measured in wet weight (WW) by researchers, which is also the preferred units for Ecopath models (Christensen and Pauly, 1993). Similar methods for estimating population numbers and biomass were used for the six sites.
(ii) Cenderawasih Bay, National Park, Indonesia. Maruanaya and Sumaryono (2023) sampled 15 Small juveniles all males with a total length ranging from 3-5 m, average taken as 3.2 m. Average weight was estimated by equation 2 at 450 kg in the Teluk Cenderawasih National Park area 13 851 km2. The bay area was estimated about 95,000 km2 larger than the marine park (see online references in Table 1 footnotes. Therefore, population number in the whole bay area was estimated at 103 = (15 × 95 000/13 851).
(iii) Raja Ampat Large juveniles reported total length 2 to 8m, so the average total length of 5.33 m was estimated by 8.0 m x 0.666 3 from the frequency distribution in Hueter et al. (2013), giving estimated average weight 2 500 kg. The study area was estimated at 46 000 km2 from Pitcher et al. (2007) who reported 143 tww whale sharks in the Raja Ampat area with production B x (P/B) of 0.003 tww/km2, so the area was calculated by 143/0.003 t/Km2 giving area = 47 667 km2, rounded to 46 000 km2.
(iv) Yucatan Larger juveniles, Reported number sampled in Gulf of Mexico 728 with area about 1 million km2 compared Yucatan reported area 116 257 km2, giving 85. The reported average total length was 6.33 m by Hueter et al. (2013), giving an estimated average weight of 3 907 kg.
(v) Sub-adults at Ningaloo marine park coral reef and open shelf water areas are about 4 000 km2 located in the southern Exmouth Plateau area of 280 000 km2. The assumed total area occupied by whale sharks is 284 000 km2. The population number was estimated using larger juveniles at Yucatan, 208 = 85*284 000/116 257. The biomass was estimated as 0.004 = ((6 063*208)/284 000)/1 000 tww/km2. Hence, the total Ningaloo area was estimated by 280 000 km2 + Ningaloo Marine park coral reef and open shelf areas ~4 000 km2= 284 000 km2. The reported average total length 7.3 m was by Norman and Stevens (2007), so the biomass 6 063 kg was estimated using equation 2.
(vi) Galapagos Breeding, fully mature adult females. Atkinson et al., 2007 appears to assume whale sharks at Raja Ampat were breeding and tentatively set a low P/B of 0.068, but Womersley et al. (2025) showed it applies to Galapagos whale sharks. Area occupied by whale sharks less than National Park at 26 300 km2, estimated from Acuña-Marrero et al. (2014). They reported number adult females 82. Size-frequency distribution female whale sharks reported as total length 9.0 to 13.1 to 14.0 m, so average taken as 11.0 m (Figure 4 in Acuña-Marrero et al., 2014), giving estimated average weight 21 444 kg.
2.2 Whale shark increase in age with total length and weight
The only published Ecopath model containing reliable whale shark ecosystem factors of biomass and production to biomass ratio, P/B, is by Ainsworth et al. (2007). As whale sharks are fish, it was realistically reasoned that the Ecopath model production to biomass ratios (P/B) could be applied to small Juveniles, large juveniles and sub-adult fish shown in Ainsworth et al. (2007). Ecopath models show P/B is highest for small juvenile fish so they can grow quickly to avoid predators. That occurs because the P/B ratio is the rate of biomass regeneration (Gascuel et al., 2008). Hence, the ratio continues to decrease with increase in size to large juveniles, sub-adult fish and is lowest for adult fish. In the Ecopath model for Raja Ampat, Indonesia by Atkinson et al. (2007), they used P/B values for Snapper, a reasonably large fish, giving a consistent decrease with size from P/B of 1.442 for small Juveniles, 1.100 large juveniles and 0.400 for sub-adult fish. They set a tentatively low P/B of 0.068 for whale sharks at Raja Ampat, apparently assuming the whale sharks were breeding adults. However, a recent study by Womersley et al. (2025) shows the P/B applies to the Galapagos adult females. They suggested the whale shark adult females may release neonate pups at Galapagos seamounts, so the value of 0.068 was applied to the Galapagos female adults. In addition, the Guénette and Morato (1997) Ecopath model at The Azores Archipelago showed fish larvae were included in zooplankton with a P/B of 5.0. That value was cautiously applied to whale shark newborn neonate pups, and tested for consistent results obtained by the other P/B values for estimation of the whale shark increase in age with weight by the doubling time method. Accordingly, those P/B values were used to estimate the relationship of age in years with total length. As the literature also provided data on the range of weight of each stage, the relationship of age with average weight was also estimated.
As mentioned above. the relationship between age in years with average total length for each area was estimated by the doubling time method by Heip (1972), who showed time to double the population, Td = ln2/r equals 0.693/r, where r is the intrinsic rate of natural increase. Accordingly, the mathematical relationships for estimation of whale shark age in years with average total length are:
Intrinsic rate (per year) r = ln(P/B +1) (3)
Doubling time (per year) Td = 0.693/r (4)
Doubling time (years) Yd = 1/Td (5)
Predicted age (years) p = Average Ls x aYd (6)
Age (years) from stage, S, to next stage, S+1, A = (average Ls x aYd ) x (Ls+1)/p (7)
Cumulative age (years) Ac = A1 + A2 + A3 + A4 + A5 + A6 (8)
The abbreviations are: Yd is the doubling time in years. Ls is average whale shark total length (m), a is the number of times Ls is multiplied by the doubling time Td, Ls+1 is the average total length in the next stage S+1, A1 is age in years neonates from age zero take to reach average age of small juvenile whale sharks, A2 age in years from small to large juveniles, etc., finally to A6 age in years from sub-adult to adult females average length (m).
The relationship of age with total length is shown in Figure 2 in the Results. The age and total length relationship shows the new born neonate stage, estimated using the P/B value of 5.0 agrees with the relationship for the other stages, indicating the neonate ecosystem conditions are reasonably described by the assumed P/B value.
It is interesting to see that although the newborn neonate pups had the highest P/B, and hence shortest Td, they had a relatively long time to reach the next stage average total length due to starting at a low total length. Likewise, adult females with the lowest P/ B had the highest number of years to increase in weight from the sub-adult length to that of the average adult female. Note that the average total lengths of all stages from neonates to sub-adult are for males and females, but for adults, the average length was used for the larger adult females.
In addition, some study areas had P/B ratios adjusted due to the reported average total length being different from that expected from the reported range in total length. For example, at Raja Ampat, Large juveniles have a P/B for large juvenile fish in Ainsworth et al. (2007) Ecopath model as 1.100 for an expected total length of about 6 m, but modified for lower whale shark average total length 5.33 m and average weight 2 300 kg, increasing P/B to 1.196 for the smaller size. At Yucatan, the larger juveniles, P/B 1.100 reduced to 0.704 for higher average total length of 6.33 m and biomass of 3 907 kg compared with the expected 5.5 m and biomass 2 500 kg.
As an example, the average weight at Yucatan estimated by equation 2 was 3 907 kg for a reported total length of 6.33 m, higher than 2 500 kg at the expected average total length of 5.5 m. That decreased P/B to 0.704=1.1*2 500/3 907. Equation 5 gave a doubling time, Yd, of 0.769 years, so multiplying by the average total length gave 6.33 × 0.769 = 4.868 m in the first year. As the average total length in the next stage at Ningaloo of 7.3 m had not been reached, the time was increased by 1.5 years to reach 7.3 m by 1.5 = 7.3/4.868, for an age increase of 2.5 years. That age was added to the accumulated ages from newborn neonates to Raja Ampat stage 3 of 6.73 years, which were estimated in a similar way, to give the next age of 9.23 years = 6.73 +2.5. All the other stages were calculated in a similar way, requiring only the average start total length multiplied by Yd with relevant adjustments. The estimated ages (years) for the six stages are shown in Table 1 and are added from the age of the first stage to the age of the next stage, and so on to the last stage, giving the total age in years.
2.3 Whale shark biological production
The biological production of fish is important for estimating the sustainable fishing mortality, which supports stability of the ecosystem (Hodgson, 2022). According to Ecopath models, biological production, P, is calculated by B x (P/B). Hence, using the above fish P/B values and estimated biomass in each whale shark area, the biological production (tww/km2/year) is shown in Table 1.
3 Results
As discussed above, the results are shown in Table 1 with explanatory notes that supplement the descriptions in the Methods. The results are used to show the following whale shark relationships: (i) average weight with average total length, (ii) cumulative ages to reach the average total length from newborn neonate pups to adult females (iii) cumulative age with average weight from neonate pups to the next stage, (iv) cumulative age with average weight from small juveniles in Cenderawasih Bay, Indonesia to adult females at Galapagos, Ecuador.
Note that due to the errors involved in estimating the average weight of the whale sharks, the values used in the following figures were rounded to whole numbers.
The relationship pf average weight with total length was initially estimated by the power equation 2 as Weight = 13.264 × L3.0811 from reliable information on the age and weight of neonate pups. The total length was estimated from the range, and in some cases using the average total length estimated by Hueter et al. (2013) by 0.6663 × maximum total length. The initial relationship was tested by investigating the relationship for all six stages in Figure 1.
The relationship obtained is:
Average Weight (kg) = 12.028 × L3.1041, R2 = 0.9991, n = 6, p < 0.001. (9)
The relationship obtained was similar to that for the neonate pups and by comparison, is similar with that by Lockyer (1976) who noted that the body weight to length relationships for large whales have the formula W = aLb, where W is body weight in tons and L is body length in m. It was found the value of b falls within the range 3.0 ± 0.6 for the whale species examined. A similar relationship was found for whales sharks that grow to about the same length as most large whales, with the exponent similar to that for large whales at 3.2118. The highly significant relationship in Figure 1 prompted examination of the age of whale sharks with increase in the reported average total length shown in Table 1. The time was estimated by the equations shown in the Methods.
The exponential relationship obtained is:
Age (years) = 1.7538 × e0.2507 x L, R2 = 0.9974, n = 6, p < 0.001. (10)
Note, the average weight of 1.5 kg at age zero indicates an age of 1.95 years to grow to average weight of small juveniles in the next stage (the next blue diamond in the regression). The consistent and highly significant relationship confirms the estimation of the values for the area occupied by the whale sharks, their average lengths, number per km2, and P/B ratios as appropriate for estimating the age increase with total length.
It was noticed the adult females took the longest time to grow to their maximum length due to their low P/B value. Surprisingly, the newborn neonates took the second longest time to reach their average weight in the next stage, apparently due to starting at a very small size.
As the age increase with total length was significant, the relationship was further tested by investigating the relationship of age in years with average weight for all six stages in Figure 3.
The relationship obtained is:
Age (years) = 0.0011 × average weight (kg) + 3.3204, R2 = 0.9592, n = 6, p < 0.001. (11)
To test the relationships without neonate pups, the five stages with estimated average weight relationship obtained is in Figure 4:
Age (years) = 0.001 × average weight (kg) + 4.5285, R2 = 0.9946, n = 5, p < 0.001. (12)
The significant relationship indicates the estimation of average age in years by equation 2, selection of ecosystem based P/B ratios for fish and the estimation of age by the doubling time method of Heip (1972) provides a wide-ranging estimation of whale shark age in years as they increase in weight to the maximum for adult females.
4 Discussion
4.1 Comparison doubling time growth with von bertalanffy growth function
The preliminary relationships obtained in Figure 1, Figure 2, Figure 3, Figure 4 are anticipated to help future research on whale shark ecology and growth rates. However, it is necessary to compare the relationships with that modelled for growth by von Bertalanffy (1938). The von Bertalanffy growth function for length with time is defined as a saturating growth curve. It is similar to the whale shark curve in obtained above in Figure 2 for whale shark age (years) with total length, which is also a saturating curve by Age (years) = 1.7538 × e0.2507 x L, except that the figure shows age increasing with length. By turning the relationship around for total length with age, Figure 5 is obtained:
|
Figure 5 Natural logarithmic relationship between estimated whale shark average total length and cumulative ages in years from newborn neonate pups to adult females |

The relationship obtained is:
Average total length (m) = 3.9945 × Ln(Age, years) – 2.2611, R2 = 0.9975, n = 6, p <0.001.
Figure 5 for whale shark total length has an initial rapid growth, levelling off over time as the fish gets larger. It is a saturating growth curve, similar to the saturating growth curve in in von Bertalanffy (1938, see their Figure 2) for length with time. The curve in Figure 5 is also similar to the growth curve obtained by Wintner (2000, see their Figure 8) for whale sharks using estimated values for L∞, K and to. Therefore, it appears the relationships obtained by the Heip (1972) doubling time, with assumed Ecopath model P/B ratios, is worthy of further research.
4.2 Environmental characteristics
At this point, the cause of whale shark occurrence in the six areas shown in Table 1 are discussed systematically in terms of the various causes of elevated zooplankton by processes such as upwelling by the Indonesian throughflow (ITF) currents around the Indonesian islands (Taufiqurrahman et al., 2020). In island archipelagos, upwelling is due to the island mass effect (Bourdin et al., 2026) and also occurs at seamounts around the Cocos Ridge at Galapagos Darwin Island (Womersley et al., 2025).
Although Syakurachman et al. (2025) reported neonate whale sharks about four months old in Saleh Bay, Indonesia, newborn neonates were found at Southwestern Taiwan by Joung et al., (1996). The pregnant female whale shark measured 10.6 m total length and weighed about 16 tonnes at full sexual maturity. That suggests large juveniles or sub-adult whale sharks migrated from Raja Ampat Papua, Indonesia through the Philippine archipelago to southern Taiwan to breed. It is likely they were after high zooplankton to support the newborn pups feeding and growth. In that regard, Hsiao et al. (2021) reported the Taiwan Bank; southern Taiwan Strait is subject to increased production by upwelling caused by the South China Sea Warm Current and the Kuroshio Branch Current. The island mass effect apparently caused bottom water to flows up onto the continental shelf, creating a high production fishing area. Note that Bourdin et al. (2026) described the Island Mass Effect (IME) as causing upwelling around islands of nutrients by water currents flowing up from deep water and increasing phytoplankton production. Therefore, increased phytoplankton production is expected to increase zooplankton abundance and presence of planktivorous fish such as whale sharks.
The Indo-Pacific Throughflow (ITF) water comes from in the Indonesian Seas is mostly from the Pacific Ocean flowing mostly above the Papua New Guinea Island from the warm west Pacific Ocean, called the Warm Pool (De Deckker, 2016). The flow enters from around the Pacific islands of Micronesia and Melanesia into the eastern Indonesian seas. From there, the water flows through the Indonesian Archipelago and is joined by warm water from the South China Sea to the Karimata Strait and Java Sea. The branches meet in the Banda Sea creating upwelling and then flowing into the eastern Indian Ocean. The ITF coming out of the Indonesian Seas flows westward across the Indian Ocean, promoting occurrence of whale sharks at the Maldives (Riley et al., 2010), Seychelles (Rowat and Gore, 2007) and north of east Africa at Gulf of Tadjoura, Djibouti (Boldrocchi et al., 2020). The majority of ITF flows south as the Agulhas current, promoting whale sharks in tropical East Africa at Mafia Island, Tanzania and Tofo Beach, Mozambique (Rohner et al., 2022). Importantly, the ITF also flows southward directly along the west coast of Australia as the Leeuwin current (Figure 1) (Taufiqurrahman et al., 2020).
The Ningaloo Marine Park and Exmouth Plateau, Western Australia attracts sub-adult whale sharks due to increased zooplankton production caused by upwelling by the Ningaloo and Leeuwin Currents. The Ningaloo Current is a northward-flowing current inshore of the Leeuwin Current, parallel to Ningaloo reef. However, the Leeuwin Current from the Indo-Pacific Throughflow causes higher nutrient concentrations than the Ningaloo Current (Vanderklift et al., 2020). Brewer et al. (2007) showed currents due to southward flow of the ITF causes increased production on the Exmouth Plateau, supported by the Dampier Ridge upwelling in the north. The Ningaloo area is at the southern end of the Exmouth Plateau and is subject to both the Leeuwin and Ningaloo current upwelling. High but variable production of zooplankton, including krill, support large planktivores, such as whale sharks and manta rays which feed on the high zooplankton abundance. It appears the sub-adult whale sharks migrate north along the Western Australia archipelago range of islands at Ashmore, Cartier and then north into the Banda Sea, Indonesia apparently looking for zooplankton areas to breed as adults.
As the Galapagos Marine Park is also in the tropical Pacific Ocean, the whale sharks were investigated for their relationship with the Indo-Pacific Throughflow, which comes from the extensive area of the tropical western Pacific islands. It was noted that fish stocks, including whale sharks, are known to migrate through the archipelago of Western and Central Pacific Islands. Importantly, the Western and Central Pacific Fisheries Commission, defines the islands as a fish migration area, including whale sharks, extending from the Micronesia islands, east of the Philippine islands, as far west as French Polynesia. The western islands are connected to the East Pacific Rise and the Galapagos Rise, containing the Galapagos Islands, and Cocos Ridge to the Isthmus connecting north and South America. As whale sharks are known to travel through the western and central Pacific islands, it is likely the study on upwelling at the islands by Helber and Weisberg (2001) is a possible reason why the whale sharks can move west from Galapagos through the Pacific islands to Indonesia. They found that although the geophysical causes of upwelling in the western Pacific islands are different from those in the central Pacific islands, the upwelling was estimated at about the same amount. Although the production of zooplankton by the upwelling is unknown in the area, it is expected the whale sharks may feed on the extensive coral reef areas around the islands that contain abundant small fish, coral related animals and potentially intermittent high-density areas of zooplankton. Significantly, the stated aim of the Commission is to ensure the long-term sustainability of highly migratory fish stocks, including whale sharks that are protected by all the island nations.
Finally, whale sharks at Yucatan in the Caribbean Sea, off the western Atlantic Ocean are abundant at times due to zooplankton production by upwelling. The study by Jouanno et al. (2018) showed zooplankton production at the Yucatan shelf is caused by wind-forced upwelling of nutrient rich water over the continental shelf. The coastal waters of the Yucatan, called the Campeche Bank, have fringing coral reefs (Aguilar-Medrano and Vega-Cendejas, 2019) that can also provide food items for whale sharks. As for the situation of whale sharks at Galapagos, it is unlikely the population in the Caribbean is isolated from other tropical areas. As they occur in the western Atlantic Ocean they may have migrated from Mozambique in southern tropical East Africa, following the productive waters of South Africa and then north along the African west coast to the Gulf of Guinea, off Angola and Nigeria (Weir, 2010). The west coast zooplankton is expected to be supported by nutrient upwelling of the Guinea Current warm water (Djakouré, 2024). Then, as shown for whales by Hodgson (2025), the whale sharks could migrate to the Caribbean Sea via the mid-Atlantic Ridge, possibly through the Cape Verde islands off the west coast of Africa. The comparison is consistent with seamounts associated with the mid-ocean ridges as important for pelagic fish and their predators. The whale sharks probably enter the Caribbean Sea through the waters off Venezuela where the highest phytoplankton and zooplankton production occurs (Mendoza, 1993; Hodgson, 2017) due to upwelling at the Venezuelan shelf (Andrade et al., 2003) and then move to the Yucatan Peninsula.
4.3 Ecosystem conditions and whale shark protection by biological production
Due to the low biological production of whale sharks in all six areas, from 0.002 to 0.011 t/km2/year, it appears all whale sharks require protection from fishing. The biological production of a fishery is important in setting the Ecosystem-Based Fishery Management, EBFM, as described by Hodgson (2022). For example, equation 5 in Hodgson (2022) shows Ppred = Qpred × √TTE, where in this case, the predator production, Ppred, is whale shark production, Qpred, is the production of zooplankton consumed by the whale sharks, and √TTE is square root of the biological production Trophic Transfer Efficiency, TTE. It was shown the TTE was estimated by TTE = 0.54 × TL-1.26, where TL is the trophic level. The whale shark TL is 3.6 ± 0.5 from fishbase (https://fishbase.se/summary/2081) gives TTE = 0.1075, which is the transfer efficiency from zooplankton production, in TL 2, to whale shark production, in TL3. The TTE of about 11% is what drives whale shark growth, as shown in Figure 2, by consumption of zooplankton. The importance of the zooplankton consumption transfer is demonstrated by the zooplankton consumption for large juveniles measured by Motta et al. (2010) at Raja Ampat, Indonesia. They found consumption averaged about 15.85 kg/day, giving 5.785 t/km2/year. Using the weighted average P/B for zooplankton of 75.9 by Ainsworth et al. (2007) in the Raja Ampat area, the estimated zooplankton production consumption is 439 t/km2/year. However, uptake by whale sharks is potentially reduced to 47.2 t/km2/year due to the TTE (47.2 = 439 × 0.1075). The approximate 90% reduction is due to respiration and defecation losses (Hodgson, 2022).
Using the ecosystem √TTE from the Ppred equation, the √0.1075 = 0.328, so the equation Ppred = Qpred × √TTE is 0.004 = Qpred × 0.328. Assuming the above data and information is correct, the net consumption of zooplankton production by whale sharks in the area, Qpred is estimated at 0.012 = (Ppred 0.004/√TTE 0.328) t/km2/year, only about 11% of the TTE of 0.1075. That overall 98.8% reduction in zooplankton production consumption from 439 t/km2/year by Motta et al. (2010) to 47.2 t/km2/year and then to about 5.27 t/km2/year (47.2 × 0.1116 {0.012/0.1075}) of explains the low biological production of the whale sharks in Table 1. The cause of the low production is not known but probably due to the long distances swam looking for zooplankton food (Hearn et al. 2016).
The low production indicates all whale sharks needing protection from fishing, as shown above applied at all the Pacific Islands. That is consistent with protection of all whales, including the large zooplankton Krill consumption by baleen whales, by Minke whales, (Balaenoptera bonaerensis), Humpback whales (Megaptera novaengliae), Fin whales (B. physalus), Right whales (Eubalaena australis), blue whale (Balaenoptera musculus) and Sei whale (B. borealis), see Reilly et al. (2004). In addition, a similar low production may apply for the zooplankton feeding manta rays and Basking sharks, so protection of those species should also be investigated.
The following further research is suggested. As the P/B ratios in Ecopath models for whale sharks are limited, it is suggested they are undertaken according to the recommended method in Christensen et al. (2005) at the following locations when whale sharks are present feeding on abundant zooplankton: The Philippine Island archipelago, Yucatan and Ningaloo coral reefs and at the long migration areas of Maldives, South-Eastern Africa, coastal South Africa, in the Guinea Current, west coast of Africa, Cape Verde Islands, as well as in the fish migration corridor of the Pacific islands. Their diet at coral reefs is important for support of their very long migration across the Pacific Ocean. Hence, research at the Pacific islands could also confirm the whale shark diet of range of coral reef plankton, found by whale shark feeding at the coral reefs around Yucatan by Motta et al. (2010) and similar findings by Rohner et al. (2013) at Mozambique and South Africa to support long-distance movements (Rohner et al. (2022).
5 Conclusions
The study findings of low biological production show the importance of protection of whale shark migrations supported by upwelling processes at open ocean seamounts and the island mass effect at tropical islands. The effect of nutrient upwelling by deep sea currents likely encourages whale shark migrations to seamount and island areas. It is hoped that these insights for the ecological basis for whale shark growth rates will be of assistance to biologists and ecosystem modellers for ongoing management of whale shark feeding and migration areas with potentially increased ecological stability of the world’s tropical ocean areas.
Funding
There was no funding for this study.
Acknowledgements
The manuscript was reviewed by an independent unknown reviewer, which led to estimation of growth rates and production, showing whale sharks require protection in all the areas examined. There was no funding for this part of the study, which developed from previous investigations of whale consumption of krill, migrations related to seamounts and ecosystem-based fishing mortalities.
Conflicts of Interest
The author declares no known conflict of interest.
Acuña-Marrero D., Jiménez J., Smith F., Doherty P.F. Jr., Hearn A., Green J.R., Paredes-Jarrín J., and Salinas-de-León P., 2014, Whale shark (Rhincodon typus) seasonal presence, residence time and habitat use at Darwin Island, Galapagos marine reserve, PLoS ONE, 9(12): e115946.
https://doi.org/10.1371/journal.pone.0115946
Aguilar-Medrano R., and Vega-Cendejas M.E., 2019, Implications of the environmental heterogeneity on the distribution of the fish functional diversity of the Campeche Bank, Gulf of Mexico, Marine Biodiversity, 49(4): 1913-1929.
https://doi.org/10.1007/s12526-019-00954-y
Ainsworth C.H., Varkey D., and Pitcher T.J., 2007, Ecosystem simulation models for the Bird's Head Seascape, Papua, fitted to data, Fisheries Centre Research Reports, 15(5): 6-172. in Pitcher, T.J., Ainsworth C.H. and Bailey, M. (eds) Ecological and Economic Analyses of Marine Ecosystems in the Birds Head Seascape, Papua, Indonesia: I. Fisheries Centre Research Reports 15(5): 184.
Andrade C.A., Barton E.D., and Mooers C.N.K., 2003, Evidence for an eastward flow along the Central and South American Caribbean Coast, Journal of Geophysical Research: Oceans, 108(C6): 3185.
https://doi.org/10.1029/2002JC001549
Boldrocchi G., Omar M., Azzola A., and Bettinetti R., 2020, The ecology of the whale shark in Djibouti, Aquatic Ecology, 54(2): 535-551.
https://doi.org/10.1007/s10452-020-09758-w
Bourdin G., Karp-Boss L., Lombard F., Gorsky G., and Boss E., 2026, Dynamics of island mass effect - part 2: phytoplankton physiological responses, Biogeosciences, 23(8): 2687-2728.
https://doi.org/10.5194/bg-23-2687-2026
Brewer D.T., Lyne V., Skewes T.D., and Rothlisberg P., 2007, Trophic systems of the North West Marine Region, Report to The Department of the Environment and Water Resources, CSIRO Cleveland, pp.156.
Cárdenas S.A., and Lew D.K., 2016, Factors influencing willingness to donate to marine endangered species recovery in the Galapagos National Park, Ecuador, Frontiers in Marine Science, 3: 60.
https://doi.org/10.3389/fmars.2016.00060
Christensen V., and Pauly D., 1993, Trophic models of aquatic ecosystems, ICLARM Conference Proceedings, 26: 390.
Christensen V., Walters C.J., and Pauly D., 2005, Ecopath with Ecosim: a user's guide, Fisheries Centre, University of British Columbia, Vancouver, November 2005 edition, 154 pp.
De Deckker P., 2016, The Indo-Pacific warm pool: critical to world oceanography and world climate, Geoscience Letters, 3(1): 20.
https://doi.org/10.1186/s40562-016-0054-3
Djakouré S., Konaté Y., Koné V., Bosson K., Koné M., and Kouadio K.Y., 2024, Relationship between the Guinea current and the coastal upwelling in northern of Gulf of Guinea, Open Journal of Marine Science, 14(4): 63-77.
https://doi.org/10.4236/ojms.2024.144004
Gascuel D., Morissette L., Palomares M.L.D., and Christensen V., 2008, Trophic flow kinetics in marine ecosystems: toward a theoretical approach to ecosystem functioning, Ecological Modelling, 217(1-2): 33-47.
https://doi.org/10.1016/j.ecolmodel.2008.05.012
Genin A., 2004, Bio-physical coupling in the formation of zooplankton and fish aggregations over abrupt topographies, Journal of Marine Systems, 50(1-2): 3-20.
https://doi.org/10.1016/j.jmarsys.2003.10.008
Guénette S., and Morato T., 2001, The Azores archipelago, 1997, Fisheries Centre Research Reports, In: Guénette S., Christensen V., and Pauly D. (eds.), Fisheries impacts on North Atlantic ecosystems: models and analyses, Fisheries Centre, University of British Columbia, Vancouver, 9(4): 241-270.
Hearn A.R., Green J., Román M.H., Acuña-Marrero D., Espinoza E., and Klimley A.P., 2016, Adult female whale sharks make long-distance movements past Darwin Island (Galapagos, Ecuador) in the Eastern Tropical Pacific, Marine Biology, 163(10): 214.
https://doi.org/10.1007/s00227-016-2991-y
Heip C., 1972, The reproductive potential of copepods in brackish water, Marine Biology, 12(3): 219-221.
https://doi.org/10.1007/BF00346769
Helber R.W., and Weisberg R.H., 2001, Equatorial upwelling in the western Pacific warm pool, Journal of Geophysical Research: Oceans, 106(C5): 8989-9003.
https://doi.org/10.1029/2000JC000401
Hodgson B., 2017, Relationships between zooplankton production, pelagic fish production and commercial finfish catch in tropical shelves, The 10th Indo-Pacific Fish Conference (IPFC10).
Hodgson B.R., 2022, An analytical solution to ecosystem-based FMSY using trophic transfer efficiency of prey consumption to predator biological production, PLoS ONE, 17(11): e0276370.
https://doi.org/10.1371/journal.pone.0276370
Hodgson B.R., 2024, Time for fishery biomass recovery from overfishing by mathematical solution of the logistic equation, European Journal of Aquatic Sciences, 3(3): 1-14.
https://doi.org/10.24018/ejaqua.2024.3.3.26
Hodgson B.R., 2025, Global importance of supporting the krill to whale component of the pelagic food web associated with migrations following deep sea seamounts, International Marine Science Journal, 1(3): 17-35.
https://doi.org/10.14302/issn.2643-0282.imsj-25-5590
Horton T.W., Palacios D.M., Stafford K.M., and Zerbini A.N., 2022, Baleen whale migration, in: Clark C.W. and Garland E.C. (eds.), Ethology and behavioral ecology of mysticetes, Ethology and Behavioral Ecology of Marine Mammals, Springer, Cham, Chapter 4: 71-14.
https://doi.org/10.1007/978-3-030-98449-6_4
Hsiao P.Y., Shimada T., Lan K.W., Lee M.A., and Liao C.H., 2021, Assessing summertime primary production required in changed marine environments in upwelling ecosystems around the Taiwan Bank, Remote Sensing, 13(4): 765.
https://doi.org/10.3390/rs13040765
Hueter R.E., Tyminski J.P., and de la Parra R., 2013, Horizontal movements, migration patterns, and population structure of whale sharks in the Gulf of Mexico and northwestern Caribbean Sea, PLoS ONE, 8(8): e71883.
https://doi.org/10.1371/journal.pone.0071883
Jouanno J., Pallàs-Sanz E., and Sheinbaum J., 2018, Variability and dynamics of the Yucatan upwelling: high-resolution simulations, Journal of Geophysical Research: Oceans, 123(2): 1251-1262.
https://doi.org/10.1002/2017JC013535
Joung S.J., Chen C.T., Clark E., Uchida S., and Huang W.Y.P., 1996, The whale shark, Rhincodon typus, is a livebearer: 300 embryos found in one 'megamamma' supreme, Environmental Biology of Fishes, 46(3): 219-223.
https://doi.org/10.1007/BF00004997
Lockyer C., 1976, Body weights of some species of large whales, Journal du Conseil International pour l'Exploration de la Mer, 36(3): 259-273.
https://doi.org/10.1093/icesjms/36.3.259
Maruanaya Y., and Sumaryono, 2023, Occurrence of whale sharks (Rhincodon typus) in the Kwatisore Waters within the Cenderawasih Bay National Park as a basis for carrying capacity estimations and assessments for ecotourism suitability, IOP Conference Series: Earth and Environmental Science, 1224(1): 012018.
https://doi.org/10.1088/1755-1315/1224/1/012018
Mendoza J.J., 1993, A preliminary biomass budget for the northern Venezuela ecosystem, in: Christensen V. and Pauly D. (eds.), Trophic models of aquatic ecosystems, ICLARM Conference Proceedings, 26: 285-297.
Motta P.J., Maslanka M., Hueter R.E., Davis R.L., de la Parra R., Mulvany S.L., Habegger M.L., Strother J.A., Mara K.R., Gardiner J.M., Tyminski J.P., and Zeigler L.D., 2010, Feeding anatomy, filter-feeding rate, and diet of whale sharks Rhincodon typus during surface ram filter feeding off the Yucatan Peninsula, Mexico, Zoology, 113(4): 199-212.
https://doi.org/10.1016/j.zool.2009.12.001
Norman B.M., and Stevens J.D., 2007, Size and maturity status of the whale shark (Rhincodon typus) at Ningaloo Reef in Western Australia, Fisheries Research, 84(1): 81-86.
https://doi.org/10.1016/j.fishres.2006.11.015
Pitcher T.J., Ainsworth C.H., and Bailey M., 2007, Ecological and economic analyses of marine ecosystems in the Bird's Head Seascape, Papua, Indonesia: I, Fisheries Centre Research Reports.
Reilly S., Hedley S., Borberg J., Hewitt R., Thiele D., Watkins J., and Naganobu M., 2004, Biomass and energy transfer to baleen whales in the South Atlantic sector of the Southern Ocean, Deep Sea Research Part II: Topical Studies in Oceanography, 51(12-13): 1397-1409.
https://doi.org/10.1016/S0967-0645(04)00087-6
Riley M.J., Hale M.S., Harman A., and Rees R.G., 2010, Analysis of whale shark Rhincodon typus aggregations near South Ari Atoll, Maldives Archipelago, Aquatic Biology, 8: 145-150.
https://doi.org/10.3354/ab00215
Robalino-Mejía C., Álvarez R., Arauz R., Cambra M., Chinchilla I., Espinoza M., García-Rada E., González-Armas R., Hearn A.R., Suárez-Moncada J., Vera A., Villalobos H., and Peñaherrera-Palma C., 2026, Characterization of pelagic assemblage on islands and seamounts of the Cocos Ridge: a regional approach for the Eastern Tropical Pacific, Marine Ecology Progress Series, 784: 1-19.
https://doi.org/10.3354/meps15127
Rohner C.A., Couturier L.I.E., Richardson A.J., Pierce S.J., Prebble C.E.M., Gibbons M.J., and Nichols P.D., 2013, Diet of whale sharks Rhincodon typus inferred from stomach content and signature fatty acid analyses, Marine Ecology Progress Series, 493: 219-235.
https://doi.org/10.3354/meps10500
Rohner C.A., Venables S.K., Cochran J.E.M., Prebble C.E.M., Kuguru B.L., Berumen M.L., and Pierce S.J., 2022, The need for long-term population monitoring of the world's largest fish, Endangered Species Research, 47: 231-248.
https://doi.org/10.3354/esr01177
Rowat D., and Gore M., 2007, Regional scale horizontal and local scale vertical movements of whale sharks in the Indian Ocean off Seychelles, Fisheries Research, 84(1): 32-40.
https://doi.org/10.1016/j.fishres.2006.11.009
Syakurachman I., Yasman Y., Putra M.I.H., Erdmann M., Patria M.P., and Setyawan E., 2025, First evidence of neonatal whale sharks (Rhincodon typus) in Saleh Bay, West Nusa Tenggara, Indonesia, Diversity, 17(12): 839.
https://doi.org/10.3390/d17120839
Taufiqurrahman E., A'an J.W., and Masumoto Y., 2020, The Indonesian throughflow and its impact on biogeochemistry in the Indonesian Seas, ASEAN Journal on Science and Technology for Development, 37(1): 29-35.
https://doi.org/10.29037/ajstd.596
Vanderklift M.A., Babcock R.C., Barnes P.B., Cresswell A.K., Feng M., Haywood M.D.E., Holmes T.H., Lavery P.S., Pillans R.D., Smallwood C.B., Thomson D.P., Tucker A.D., Waples K., and Wilson S.K., 2020, The oceanography and marine ecology of Ningaloo, a world heritage area, Oceanography and Marine Biology: An Annual Review, 58: 143-178.
https://doi.org/10.1201/9780429351495-4
Von Bertalanffy L., 1938, A quantitative theory of organic growth (inquiries on growth laws II), Human Biology, 10(2): 181-213.
Weir C.R., 2010, Sightings of whale sharks (Rhincodon typus) off Angola and Nigeria, Marine Biodiversity Records, 3: e50.
https://doi.org/10.1017/S1755267209990741
Wintner S.P., 2000, Preliminary study of vertebral growth rings in the whale shark, Rhincodon typus, from the east coast of South Africa, Environmental Biology of Fishes, 59(4): 441-451.
https://doi.org/10.1023/A:1026564707027
Womersley F.C., Waller M.J., and Sims D.W., 2025, Do whale sharks select for specific environments to give birth?, Ecology and Evolution, 15(2): e70930.
https://doi.org/10.1002/ece3.70930
. HTML
Associated material
. Readers' comments
Other articles by authors
. Bruce Hodgson

Related articles
. Whale shark growth rates
. Breeding areas: Seamount upwelling
. Island mass Effect: Tropical ocean migrations: Ecopath model ecosystem conditions
Tools
. Post a comment